Terrible science writing in The Skeptic magazine.

Speaking of misleading headlines, The Skeptic, which is a fine publication produced by Australian Skeptics and which, to my knowledge, does not itself contain any terrible science writing, has reprinted my blog post Anatomy of a Bad Science Story as an article in the latest issue (with permission, of course).

Have a look, and if you’re in the Land of Oz (or, presumably, anywhere), why not join Australian Skeptics and get the full magazine on a regular basis?

Click for full size view.

This just in: DNA barcoding is not the be all and end all of the universe.

I want to share a few quotes about DNA barcoding. Some of these are from critics of barcoding (Roe and Sperling 2007) and some are from proponents of DNA barcoding (Hebert and Gregory 2005). For fun, see if you can guess which is which, and then see if you can guess why critics keep saying the same thing despite what barcoding actually involves.

This shortfall suggests that mtDNA is not as universally successful as suggested by DNA-barcoding advocates. Additional markers are clearly essential to clarify species boundaries, providing additional support for an integrative, multilocus approach to delimiting species.

There is an important distinction between “describing” and “delimiting” species, but a conflation of the two has created uneasiness about the use of DNA barcodes as the foundation of future taxonomic descriptions. We emphasize that DNA barcoding seeks merely to aid in delimiting species – to highlight genetically distinct groups exhibiting levels of sequence divergence suggestive of species status. By contrast, DNA barcodes – by themselves – are never sufficient to describe new species. At some stage, clearly divergent DNA barcodes, in combination with other information, will be used as the basis for providing a new Linnaean name and, as with any taxonomic hypothesis, this would be subject to ongoing re-evaluation. For example, in a recent survey of North American birds, the threshold for delineating probable new species was arbitrarily set at 10x the average within-species variation of the entire barcode dataset. This led to the revelation of four presumptive new species, but decisions regarding the formal recognition of these taxa are left, appropriately, to the ornithological community (notably, existing morphological and behavioural information supports these new hypotheses).

Rather than concentrating on a single character type (e.g. morphological or DNA sequence variation), a wide range of characters, including molecular data, morphology, behaviour, and geography, are integral to assessing species boundaries and delimiting species.

DNA barcoding using a single gene region does not assure complete taxonomic resolution, but it does promise proximity. Based on past results for varied animal groups, DNA barcoding will deliver species-level resolution in 95-97% of cases. When it fails, it will narrow the options to a small number of congeneric taxa (which, in many cases, could be resolved fully with additional genetic or other data).

Additional sources of data, such as morphology, host preference, geographic range and pheromone can be used when elucidating species boundaries, as this approach will improve detection of incongruence between markers, allowing insight into the process of speciation.

The synergy between DNA barcoding and studies of morphological/ecological diversity is further illustrated by the case of the skipper butterfly, Astraptes fulgerator, in which a combined morphological, natural history and barcoding approach revealed a complex of 10 species in one small area of Costa Rica. Importantly, several of these species showed a relatively small barcode divergence, but a coupling of this information with records on larval host plants and morphology illuminated the full diversity of the complex.

_________

References

Hebert, P.D.N. and T.R. Gregory. 2005. The promise of DNA barcoding for taxonomy. Systematic Biology 54: 582-859.

Roe, A.D. and F.A.H. Sperling. 2007. Population structure and species boundary delimitation of cryptic Dioryctria moths: an integrative approach. Molecular Ecology 16: 3617-3633.

Welcome to Mobile DNA blog.

When I began this blog, several of the big-name bloggers were kind enough to point people in my direction. While Genomicron is not in the same league as, say, Pharyngula or Sandwalk, it has become reasonably well established. As such, it could provide at least some help to new bloggers if I make a note of their new blogs.

Case in point, Mobile DNA by Prof. Cedric Feschotte (University of Texas at Arlington). There are few things cooler in genomics than transposable elements (in my humble opinion), and this is the subject of both Prof. Feschotte’s research and his neonate blog. Let’s give him some hits so that he will be encouraged to continue sharing his insights on this topic with the rest of the blogosphere.

If anyone else has started a new blog about genomics or evolution, feel free to link to it in the comments.


Bloggers for Peer-Reviewed Research Reporting (BPR3): Why I won’t be participating (yet?).

I am partially aware of the discussions that have been taking place about having some sort of quasi-official designation that a particular blog post is discussing peer reviewed research. I am all for improving the discourse on blogs when it comes to reporting research. Some readers may recall that I was involved in a minor row (since resolved amicably) over the way a discussion of a paper by some well respected researchers was conducted. I also don’t think blogs count as anything like peer review, and if anyone suggests otherwise, it’s probably because they don’t actually participate much in the peer review process as either an author or a reviewer.

On the other hand, I think blogs are an excellent place to discuss, disseminate, and dissect peer-reviewed articles in a way that makes them more accessible to a broader audience and opens the scientific process to view by non-specialists. My concern is simply that people could mistake what happens on blogs for how the peer review system functions.

There is now a new icon that bloggers are encouraged to use when discussing peer-reviewed research, which was the victor in an open design contest by the Bloggers for Peer Reviewed Research Reporting (BPR3):

According to their site,

Bloggers for Peer-Reviewed Research Reporting strives to identify serious academic blog posts about peer-reviewed research by developing an icon and an aggregation site where others can look to find the best academic blogging on the Net.

I agree with the general notion of letting readers know that peer-reviewed research (vs., say, just someone’s opinion) is being described, but I’m afraid I can’t participate in the program as structured. Why? Because the name, “Bloggers for Peer Reviewed Research Reporting” is ambiguous — is the reporting peer reviewed? No, it isn’t, but this could give the wrong impression. In fact, the logo strongly reinforces this, reading only “Peer Reviewed Research BPR3“.

It’s a decent idea, but the impression it gives in its current manifestation is contrary to my views on the role of blogging in scientific communication.

_______

Update:

Evolgen is promising (threatening?) to publish original, unreviewed research on a blog. Slap the above icon on it, and this would give a very misleading impression to nonexperts. I have to oppose both developments if they are going to, in any way, appear to circumvent or undermine peer review processes. (Update: he will be using this as an educational demonstration, which I fully support… but let’s not have it go beyond that on other blogs).

BPR3 has provided a reply to this post and the comments it engendered, and to their credit they are looking at making some changes to improve the situation. Of course I will be open to participating in the future if I feel it is useful and in accordance with my views on blogging about science. I wish them luck with this.


Genomicron discovers Adaptive Complexity, and likes it.

Via Panda’s Thumb, I have come across a blog that I wish I had known about sooner. It is Adaptive Complexity by Michael White, postdoc in the Department of Genetics and the Center for Genome Sciences at the Washington University School of Medicine, who is also a featured writer at Scientific Blogging (some readers may recall that I was invited to be a featured writer, but I ultimately decided not to commit due to time constraints).

In any case, Adaptive Complexity provides some good posts, and expresses some of the same frustrations as I do, about non-coding DNA. Some highlights:

Welcome to my blogroll and feed reader, Dr. White.


Favourite science blogs.

As noted by, well, everybody, The Scientist is assembling a list of the bioblogosphere’s best. Here is my list of favourite blogs — this isn’t exhaustive, however, as there are many that I read regularly in addition to this (see my blogroll for more). These are just the ones that I follow most closely.

  • Pharyngula — PZ Myers’s monster chimaera between hardcore objective science and stinging anti-theism.
  • Sandwalk — Online home of Larry Moran, everyone’s favourite curmudgeonly Canuck.
  • The Loom — Proof courtesy of Carl Zimmer that science writing can be consistently top-notch.
  • Evolution…Not Just a Theory Anymore — Although I don’t care for the name (evolution will always be both a fact and a theory), Greg Laden continually offers excellent insights.
  • ERV — Sarcastic, merciless, and never boring, and she knows a heck of a lot about ERVs and HIV.
  • John Hawks Weblog — Interesting, accessible discussions about things anthropological.
  • Aetiology — Tara Smith’s launching pad for discussions on evolution and health.
  • Evolgen — Thoughts on evolutionary genetics from a grad student who knows his material.
  • Laelaps — Home of Brian Switek, one of the hardest working bloggers around, who produces top quality essays on important topics in evolutionary science.
  • The DNA Network — A great collection of blogs on the subjects of genetics, genomics, and medicine. Features great blogs like Eye on DNA, My Biotech Life, and ScienceRoll.
  • Sex, Genes & Evolution — John Logsdon’s blog about, well, sex, genes, and evolution; great stuff, and I wish there were more frequent posts.
  • Interrogating Nature — High end contributions from Chris Harrison, a bright, young scientist-in-training.
  • The Tree of Life — Genomics plus opinions from Jonathan Eisen, good stuff.
  • Barcode of Life Blog — Superb clearinghouse by Mark Stoeckle on information regarding the ever-expanding Barcode of Life initiative.
  • EvolutionBlog — Plenty of interesting insights from Jason Rosenhouse on evolution.

By the way, if you like this blog, please be sure to post a comment about it on The Scientist‘s site!


On the lookout for DAPs!

Larry Moran and PZ have both picked up on the term “DAP“. There have already been several more examples identified outside the realm of genomics in their comments threads. As such, I think that “DAP” can be given the following broadened definition:

Dog’s Ass Plot (DAP, or Dapper):

A graphical representation of data in any field that, through a lack of clear axis labels, selective inclusion/exclusion of data, visual presentation style, and/or other questionable characteristics, generates a misleading interpretation of the data in the viewer, especially by implying an illusory pattern that is not supported by the available data.

Can you indicate an example from your own subject of study? If so, please provide a link in the comments section. Bring on the Dappers!!


The tale of the Matrix Beetle.

Gather ’round, and I will tell you the tale of the Matrix Beetle.

It began in England — London, to be precise — during the second half of my two-year NSERC postdoc. I had spent the first year in New York at the incredible American Museum of Natural History, and decided to spend the second in the UK at the equally remarkable Natural History Museum. Time well spent in both cases. In London, I joined the lab of Alfried Vogler, an expert on tiger beetles, accomplished molecular systematist, and all-around excellent person. Alfried is, like many of my colleagues, interested in the applications of molecular tools to the problem of identifying the probable 10 million species on the planet. He takes it a step farther in some cases and would like to see a “DNA taxonomy” and not just “DNA barcoding” (there is a big difference, folks), but the basic point remains that he is interested in exploring how modern genetic methods can inform the identification of life.

Every Friday at the NHM, people would gather for inexpensive (by UK standards), though certainly not cheap, beer; it was here that I discovered Leffe, which, to my delight, is also available in Canada (at the LCBO, not the Beer Store, in case you’re looking for it in Ontario). One evening whilst enjoying said brew, Alfried remarked that someone in the lab had shown him a DNA sequence that morning, and that he had looked at it and said “That’s not from a tiger beetle”. He then noted — jokingly, of course — that if he had seen the real beetle he may not have been so sure. “What are you, like the Matrix?,” I snorted, “You just see DNA sequences raining down all over?”.

Deciding to follow up on this amusing notion, I created an image of a tiger beetle as seen in a Matrix world of DNA sequences. I put this on the computers in the lab, and hilarity ensued. Someone joked that it would be funny if we managed to get that on a journal cover. I agreed, but left it at that.

For those of you who follow the literature, you’ll know that there is a vocal opposition to DNA barcoding. Most of this comes from (some) taxonomists who see barcoding as a threat to their discipline. A debate on this issue was held at the PEET meeting in 2004 (watch the video), with a follow-up “discussion” to be held in the pages of Systematic Biology. By this time, I was back in Guelph, and Paul Hebert and I were neck deep in writing a multi million dollar Genome Canada grant (which, incidentally, took exactly $0.00 from the pockets of taxonomists and delivered a sizable chunk of funds to many non-molecular types). As a result, Paul was regretfully planning to withdraw from submitting his paper to the journal issue. I thought this would be a mistake, busy though he was, because it would have let the anti-barcoding side have the only word. We agreed to work on the paper together, which consisted of answering a series of questions that had arisen from the PEET meeting.

When the papers were accepted, the journal editors asked if anyone had ideas for a cover image. On a lark, I sent in the “Matrix Beetle” — and they wanted it.

And so, from the beer gardens of the NHM to the cover of Systematic Biology Volume 54 Number 5, I give you… the Matrix Beetle:
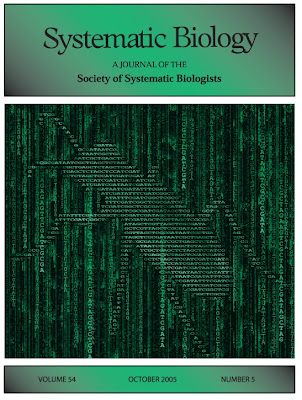
Cover Illustration: The recent proposal to use short, standardized gene sequences as unique identifiers of species – known as DN barcoding – has generated both strong support and vocal opposition in certain biological circles. The potential impact of DNA barcoding as either a help or a hindrance to taxonomic research represents an especially polarizing point of contention. A debate on the issues of DNA barcoding was held at the fifth biennial conference of the Partnerships for Enhancing Expertise in Taxonomy (PEET) in September 2004 at the University of Illinois at Urbana-Champaign. The debate was moderated by Vincent Smith, and involved Paul Hebert, the lead proponent of DNA barcoding, and Kipling Will, a vocal barcoding opponent. As a follow up to this debate, two contrasting position papers dealing with DNA barcoding are provided in this issue, moderated once again by a contribution from Smith. On the pro-barcoding side, Hebert and Gregory outline what they consider to be the beneficial aspects of DNA barcoding for taxonomy and other biological disciplines, where as Will et al. provide an opposing perspective in which they argue that DNA barcoding will be detrimental to taxonomic science. Neither set of authors has been permitted to read the others’ contribution prior to publication. Image © 2005 by T. Ryan Gregory.
Discovery wants to "demote" fungi.

Here’s an interesting story from the Discovery Channel.

Plants and animals: long lost relatives?

“Yes,” I know you’re thinking, “next question?”.

But wait, the story takes a different approach.

Plants and animals may occupy distinct branches on the tree of life, but they could be more alike than we think.

In fact, green plants and animals enjoy a relatively close evolutionary relationship that has been obscured by a narrow focus on DNA sequences to find relatedness, says biologist John Stiller of East Carolina University.

Plants, fungi and animals are all in a group called the eukaryotes — distinguished by their advanced cellular machinery. But some eukaryotes, most notably the fungi, have long been considered more closely related to animals than plants are.

Stiller’s theory suggests organisms such as fungi should be given a demotion — placed further from animals on the tree — while green plants should get a leg up.

Say again???

Another attribute shared by plants and animals, according to Stiller, is the way the genetic material RNA operates in both groups. In both plants and animals, RNA acts as an intermediary between DNA and the protein it codes for. The enzymes that put RNA to work in a cell are similar in plants and animals, but not present in fungi or other organisms, he said.

It is, of course, utterly inconceivable that the common ancestor to all three groups had this trait which was then lost in fungi. Because fungi are, of course, not a derived group that has been evolving for exactly the same amount of time as plants and animals by definition. Oh no.

Maybe the paper makes a good argument. Maybe plants and animals are sister taxa to the exclusion of fungi. But one thing’s for sure — no one’s getting “demoted” one way or another because this idea of rank was should have been abandoned 150 years ago.

______
Update:

See Sex, Genes & Evolution for more insights on the actual hypothesis, which should not be judged on the basis of how it was reported in the press.


Proof that introns are functional… come again?

I use Google Reader to aggregate not just blogs but science news, journal contents, and index searches. The feed for my weekly PubMed search turned up a real doozy. The record had been deleted by the time I got to PubMed, although I did manage to track it down.

Check this one out, it’s the zaniest abstract I have seen in some time:

The Genomic Structure: Proof of the Role of Non-Coding DNA
Bouaynaya, N. Schonfeld, D.

Engineering in Medicine and Biology Society, 2006. EMBS ’06. 28th Annual International Conference of the IEEE, Aug. 2006, pp. 4544-4547.

We prove that the introns play the role of a decoy in absorbing mutations in the same way hollow uninhabited structures are used by the military to protect important installations. Our approach is based on a probability of error analysis, where errors are mutations which occur in the exon sequences. We derive the optimal exon length distribution, which minimizes the probability of error in the genome. Furthermore, to understand how can Nature generate the optimal distribution, we propose a diffusive random walk model for exon generation throughout evolution. This model results in an alpha stable exon length distribution, which is asymptotically equivalent to the optimal distribution. Experimental results show that both distributions accurately fit the real data. Given that introns also drive biological evolution by increasing the rate of unequal crossover between genes, we conclude that the role of introns is to maintain a genius balance between stability and adaptability in eukaryotic genomes. (Emphasis added, in case that didn’t leap out at you already).

There you have it. Introns are ingenious decoy targets, and some fancy math PROVED it. As if a few pages of equations weren’t enough, they even provided a basic analysis of exon sizes in three species — and one wasn’t even a mammal. Sadly, no Dappers though.